

A chloroplast is a specialized membrane-bound organelle found in plant cells and many algal cells, with a major role in photosynthesis. It is one of the plastids, and not simply the “green part” of the plant cell. Plastids are specialized organelles found in plant and algal cells and can perform different functions such as food synthesis, storage, and pigment-related functions. Chloroplasts are the green plastids used in photosynthesis.
The chloroplast is made up of an outer and inner membrane, while within it is the stroma and an internal membrane system forming the thylakoids. These thylakoids contain the photosynthetic pigments. Chlorophyll is one of these pigments, giving the plant its green colour and absorbing light energy used during photosynthesis.
Chloroplast and chlorophyll are not the same, it is a complete organelle, while chlorophyll is the green photosynthetic pigment mainly associated with the thylakoid membranes inside the chloroplast.
Where Chloroplasts Are Found?
Chloroplasts are mainly found in the green and photosynthetic cells of plants and algae. In higher plants, they occur most abundantly in leaves, particularly in the mesophyll tissue. They are also present in several other green parts of plant.
The following are the major sites where chloroplasts are found-
- Chloroplasts are present in the photosynthetic cells of green plants, including lower and higher plants. Their number and development may vary according to the type of cell.
- In leaves, chloroplasts are found in large number in the mesophyll cells. This is the major photosynthetic tissue of the leaf and contains most of the chloroplast population.
- They are also found in green stems and other chlorenchymatous tissues. Chloroplast development can take place in different green tissues of the plant, not only in leaves.
- Guard cells surrounding the stomata also contain chloroplasts. Their number is generally much smaller than that present in the mesophyll cells.
- Chloroplasts are present in photosynthetic algae also. In these eukaryotic algae, chloroplast may occur in different forms and arrangements within the cell.
- They can also occur in some embryo cells and other green developing tissues. During plant development, proplastids present in such cells may develop into mature chloroplasts when the tissue becomes photosynthetic.
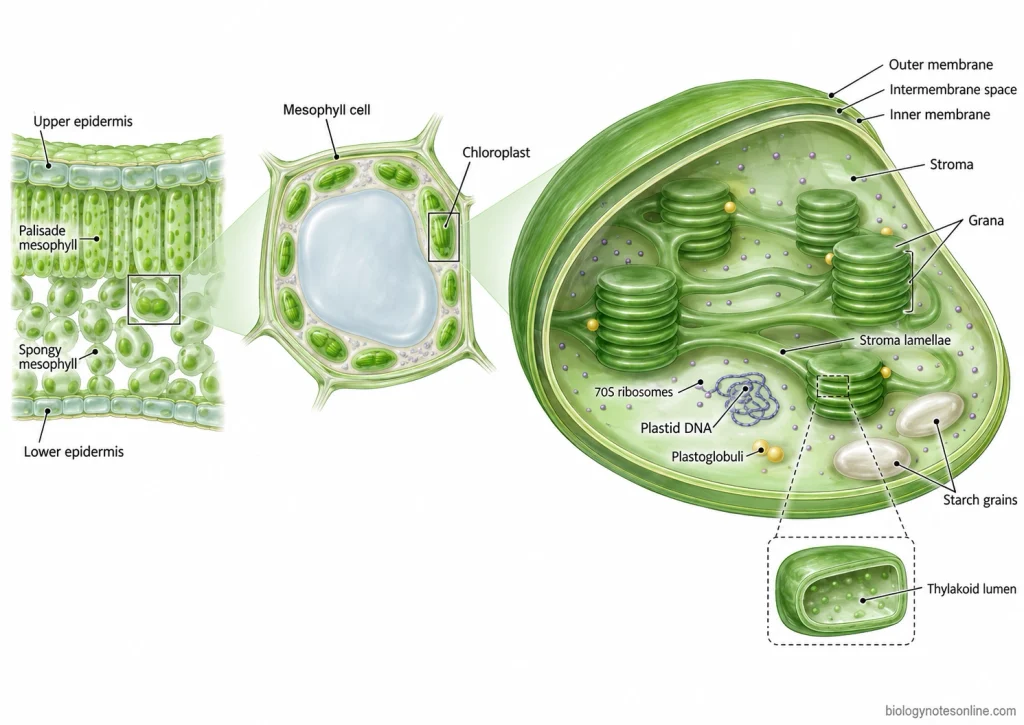
Structure of Chloroplast
Chloroplast is a double membrane-bound plastid, containing an internal membrane system called thylakoids. The internal matrix is called stroma. Different structures like grana, stroma lamellae, DNA, ribosomes, starch grains and plastoglobuli are present within it.
The following are the major structural parts of chloroplast-
- Chloroplast envelope- It is the double membrane covering present around the chloroplast. The envelope is made up of an outer membrane and an inner membrane, with a small intermembrane space between them.
- Outer membrane- The outermost covering of chloroplast. It is comparatively permeable to different small molecules.
- Inner membrane- It is present just below the outer membrane and encloses the stroma. Different transport proteins are present in this membrane, which are used for movement of substances into and out of chloroplast.
- StromaStroma is the fluid matrix of chloroplast enclosed by the inner membrane. It contains different enzymes, chloroplast DNA, RNA, 70S ribosomes, starch grains and other soluble substances.The enzymes required for carbon fixation are also present here.
- Thylakoids- These are flattened, membrane-bound sacs present in the stroma. The thylakoid membrane contains chlorophyll, photosystems and the electron carriers required for light reaction.A space is enclosed inside each thylakoid. This is referred to as thylakoid lumen.
- Grana- The thylakoids are arranged one above another in the form of stacks. Each stack is called a granum and several such stacks are called grana.Photosystem II (PSII) is mainly present in the stacked thylakoid regions.
- Stroma lamellaeThe grana are connected with one another by unstacked thylakoid membranes. These membranes are called stroma lamellae or intergranal lamellae.Photosystem I (PSI) and ATP synthase are mainly found in these unstacked regions.
- Thylakoid lumen- It is the internal cavity of thylakoid. During light reaction, hydrogen ions (H⁺) are accumulated in the lumen and later used for ATP formation.
- Chloroplast DNA- Chloroplast contains its own DNA in the stroma. The DNA occurs in regions called nucleoids. It carries genes for some proteins and RNA molecules of chloroplast.
- Ribosomes- The ribosomes present in chloroplast are 70S type. They are involved in synthesis of proteins encoded by chloroplast DNA.
- Starch grains– Starch grains are found in the stroma as temporary storage bodies. They contain the carbon stored from photosynthesis.
- Plastoglobuli- These are small lipid-containing bodies found associated with thylakoid membranes. They contain different lipids and compounds taking part in plastid metabolism.
Photosynthetic Pigments and Protein Complexes of Chloroplast
Photosynthetic pigments of chloroplast are present in the thylakoid membrane, where most of them occur in association with proteins. These pigments absorb light required for photosynthesis. Some are also involved in protection of the photosynthetic apparatus from excess light.
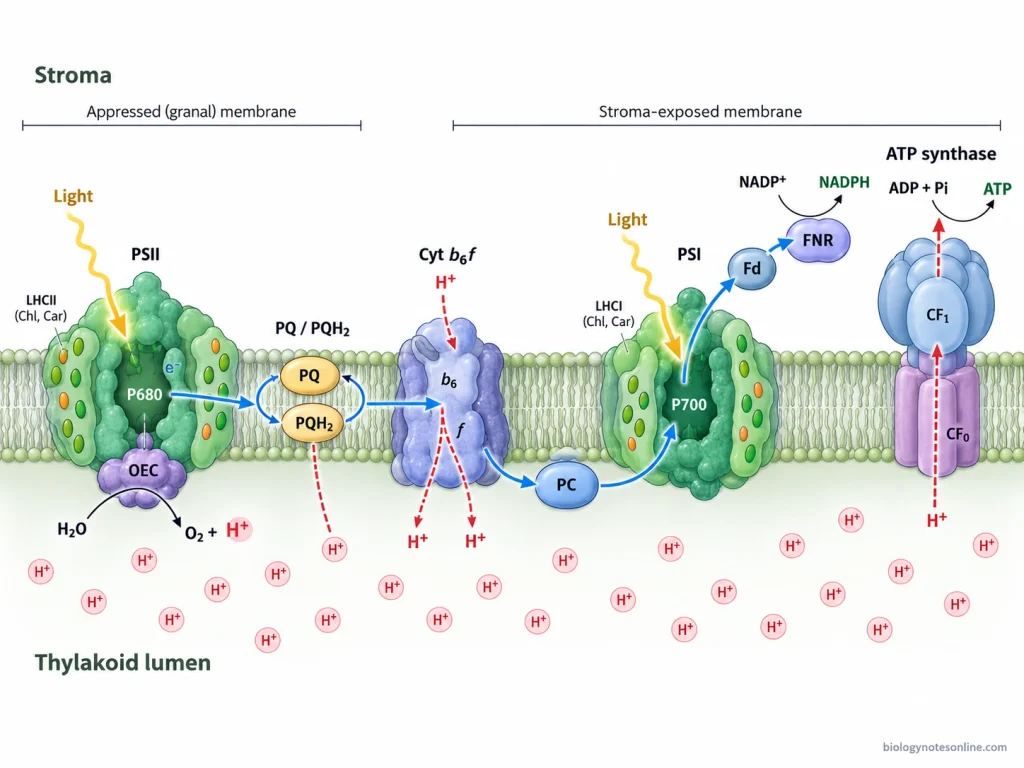
The major pigments and protein complexes are as follows-
- Chlorophyll a– Major photosynthetic pigment of plants. It is present in the antenna complexes as well as in reaction centres of both photosystems. In Photosystem II, the special reaction centre chlorophyll is P680. Photosystem I contains P700. These chlorophyll molecules directly take part in the primary photochemical reactions.
- Chlorophyll b– It is an accessory photosynthetic pigment, occurring mainly in the light-harvesting complexes of higher plants. Chlorophyll b absorbs somewhat different wavelengths of light than chlorophyll a. Thus, more range of light can be collected by the photosynthetic system and its excitation energy is transferred towards the reaction centre chlorophyll.
- Carotenoids– These are yellow to orange accessory pigments of the chlorophyll-protein complexes. Carotenes (e.g., β-carotene) and different xanthophylls are included under carotenoids. Light harvesting is one of their functions. They also have a major role in photoprotection. During strong illumination, excess excitation energy and harmful reactive species are reduced by carotenoid-dependent protective processes.
- Light-Harvesting Complexes (LHCs)– Chlorophylls and carotenoids are arranged with proteins forming these pigment-protein complexes. A large number of pigment molecules together make an antenna system. The light energy is first collected here and then passed on to the reaction centre. LHCII is mainly associated with Photosystem II, whereas LHCI forms the antenna of Photosystem I.
- Photosystem II (PSII)– It is a large pigment-protein complex embedded within the thylakoid membrane. P680 chlorophyll a forms the reaction centre. D1 and D2 are the core proteins, while CP43 and CP47 act as inner antenna proteins. Water oxidation takes place in PSII by the oxygen-evolving complex (OEC) containing a Mn₄CaO₅ cluster. During this process, electrons and protons are released. Molecular oxygen (O₂) is formed. The electrons are then passed to plastoquinone.
- Cytochrome b₆f complex– Between Photosystem II and Photosystem I is the cytochrome b₆f complex. Reduced plastoquinone (plastoquinol) supplies electrons to this complex, which are further transferred towards plastocyanin. mAt the same time, protons are released into the thylakoid lumen. This produces the proton gradient required for ATP formation.
- Photosystem I (PSI)– P700 is its reaction centre chlorophyll. Electrons coming through plastocyanin enter the Photosystem I and after absorption of light, these are again raised to a higher energy level. mFrom here, electrons move through different electron acceptors and finally reach ferredoxin (Fd). Ferredoxin-NADP⁺ reductase (FNR) uses these electrons for reduction of NADP⁺, forming NADPH.
- Chloroplast ATP synthase– This complex occurs in the thylakoid membrane. It has a membrane-associated CF₀ region and catalytic CF₁ region. mIts functioning is based on the proton gradient across the thylakoid membrane. H⁺ passes from thylakoid lumen back towards the stroma through ATP synthase. During this movement, the energy is utilized for synthesis of ATP from ADP and inorganic phosphate (Pi).
Chloroplast Semi-Autonomy and Biogenesis
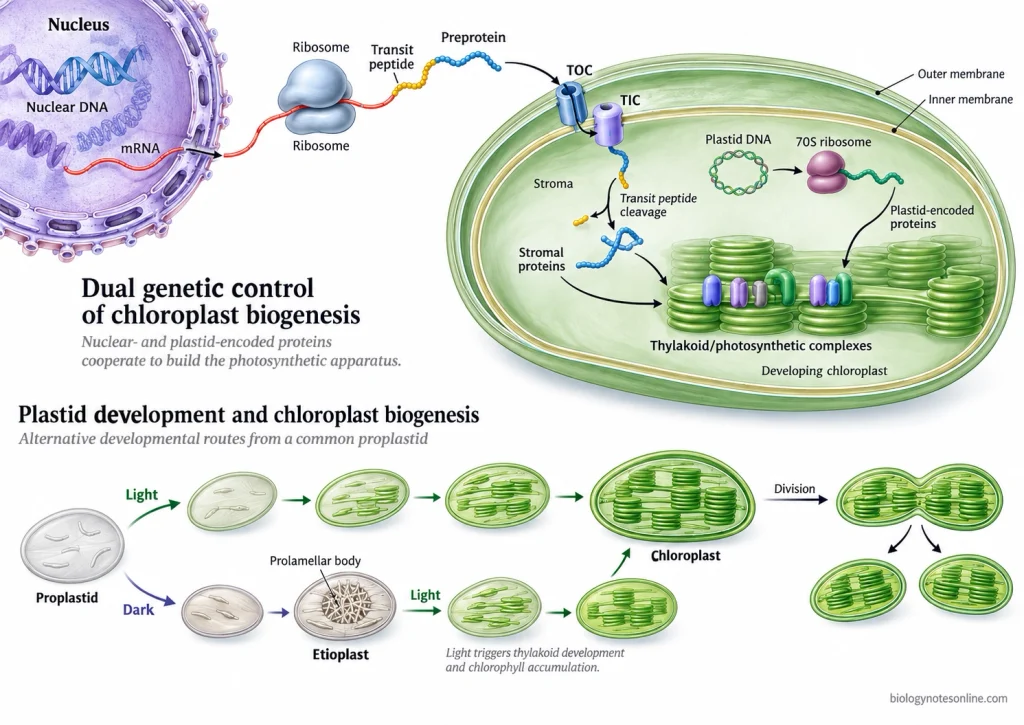
Chloroplast Semi-Autonomy
Chloroplast is a semi-autonomous organelle because it contains its own DNA and bacterial-type 70S ribosomes. It can synthesize some of its proteins by itself. However, most of the proteins required by chloroplast are encoded by nuclear genes and formed in the cytosol. Thus, chloroplast is not completely independent.
The functioning of chloroplast therefore depends upon both chloroplast genome and nuclear genome. This is referred to as its “semi-autonomous nature”.
Chloroplast Biogenesis
Chloroplasts are not formed de novo. They develop from already existing plastids, mainly proplastids present in meristematic tissues. The process involves development of internal membranes, formation of photosynthetic components, protein import and finally chloroplast division.
The following are the major steps involved in chloroplast biogenesis-
Step 1- Development of proplastid
Proplastid is a small and undifferentiated plastid from which chloroplast develops. In the presence of light, proplastid starts changing into chloroplast.
Under dark condition, however, an etioplast can be formed first. When exposed to light, the etioplast further develops into chloroplast.
Step 2- Activation of chloroplast development
Light acts as an important signal in chloroplast development. Genes required for the process are now expressed from both nuclear genome and plastid genome.
The plastid has its own transcription and translation system. But a large number of proteins required during development are controlled by nuclear genes.
Step 3- Import of nuclear-encoded proteins
Most chloroplast proteins are synthesized outside the chloroplast in cytosol as precursor proteins. These generally contain an N-terminal “transit peptide” which directs them towards chloroplast.
The proteins are transported through the outer and inner chloroplast envelope by TOC and TIC complexes, respectively. After entering the chloroplast, the transit peptide is removed. The proteins are then transported to their required sites.
Step 4- Formation of thylakoid membrane
The internal membrane system of proplastid is poorly developed. During this process, membrane lipids, proteins and pigments begin to build up.
The thylakoid membrane system is formed. These membranes further become organized into grana and stroma thylakoids.
Step 5- Chlorophyll formation and assembly of photosynthetic components
Chlorophyll is formed and photosynthetic proteins start accumulating in the developing thylakoid membrane. Photosystem I (PSI), Photosystem II (PSII), cytochrome b6f complex and ATP synthase are assembled.
Their components are supplied by both nuclear and plastid genetic systems.
Step 6- Formation of mature chloroplast
With the development of thylakoid membrane and photosynthetic machinery, the plastid becomes green and photosynthetically functional. A mature chloroplast is now formed.
Still, a large part of its proteins continue to come from nuclear genes.
Step 7- Chloroplast division
The number of chloroplasts is increased by division of already existing plastids. FtsZ and other division proteins take part in formation of the division machinery.
The chloroplast becomes constricted and finally separates into daughter plastids. It is a fission-like process.
Origin and Evolution of Chloroplasts
Chloroplasts are believed to have developed from an ancient cyanobacterium that entered into a primitive eukaryotic cell and remained inside it. This association became permanent with time and the cyanobacterial cell was converted into a photosynthetic organelle. During this process, many genes were lost or shifted to the host nucleus, while some bacterial characters were still retained in chloroplasts.
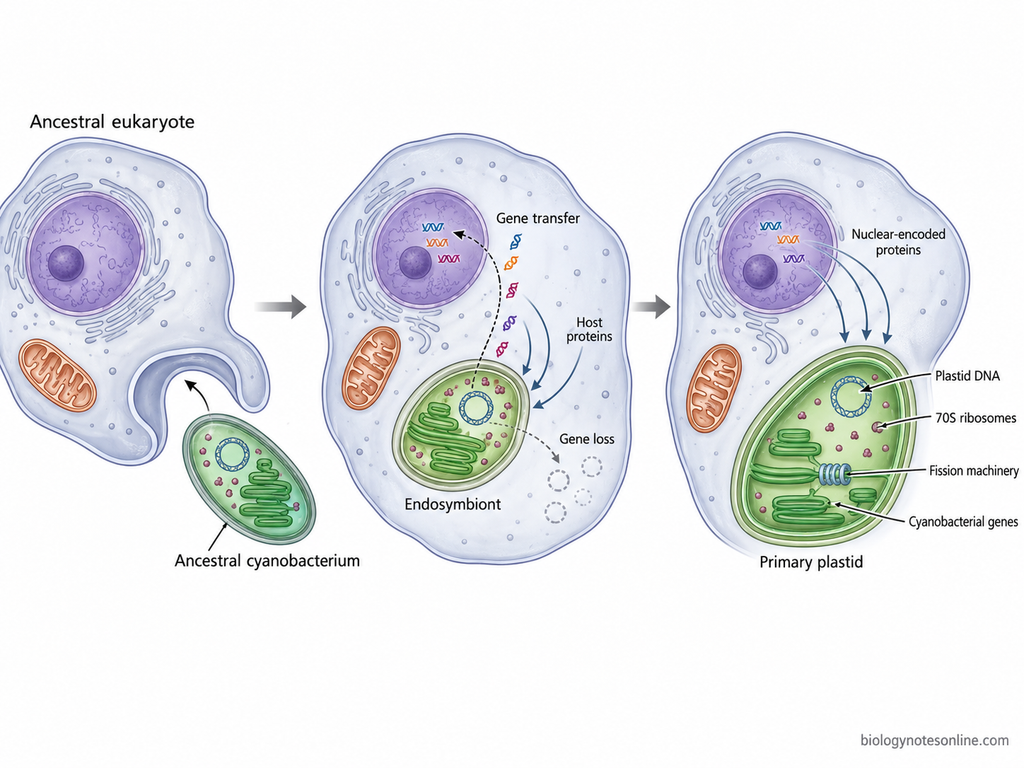
Endosymbiotic Origin
- The origin of chloroplast is explained by the endosymbiotic theory.
- According to this theory, an ancestral eukaryotic cell engulfed a photosynthetic cyanobacterium. Instead of being digested, the cyanobacterium remained within the host cell and continued its photosynthetic activity.
- The association was beneficial to both. The cyanobacterium supplied photosynthetically fixed carbon, while the host provided a protected cellular environment and other required substances.
- With prolonged association, the cyanobacterium gradually lost its independent nature. Many cellular functions were lost, some were controlled by the host, and finally it became a permanent cell organelle.
- Plastids formed directly by this cyanobacterial uptake are known as primary plastids. They are present in green plants and green algae, red algae and glaucophytes.
- Molecular studies show that these plastids have a common relationship with cyanobacteria. However, the exact present-day cyanobacterial lineage from which the plastid ancestor developed is still not clearly fixed.
- In some algae, plastids were acquired later when one eukaryotic cell engulfed another photosynthetic eukaryote already carrying a plastid. This is referred to as secondary endosymbiosis. Tertiary endosymbiosis is found in a few groups where another level of plastid-containing cell uptake occurred.
Evidence for Endosymbiosis
The following are some of the important evidence supporting the cyanobacterial origin of chloroplasts-
- Presence of chloroplast DNA- Chloroplasts possess their own genome. It is much reduced in size compared to a free-living cyanobacterium, but several genes retained in the plastid show cyanobacterial relationship.
- During the evolution of chloroplast, a large number of genes of the original endosymbiont were lost. Many others moved into the nuclear genome of the host cell. Thus, the present chloroplast genome represents only a small part of the genome once present in its cyanobacterial ancestor.
- Bacterial type translation machinery- Chloroplasts contain their own ribosomes and different components required for translation. The ribosomes are generally 70S type, similar to bacterial ribosomes and smaller than the cytoplasmic 80S ribosomes of eukaryotic cells.
- Chloroplasts also contain plastid rRNAs and some proteins required for their own protein synthesis. This bacterial-related translation system is one of the important characteristics retained from the ancestral endosymbiont.
- Division of chloroplast- Chloroplasts are produced from pre-existing plastids by division. The process contains several proteins having bacterial origin.
- One of them is FtsZ, an important division protein related to the bacterial cell division system. MinD and MinE are also bacterial-related components involved in plastid division, although modern chloroplast division is not completely bacterial and it also uses proteins developed or supplied by the eukaryotic host.
- Molecular phylogeny- Comparison of plastid rRNA, plastid proteins and genes of cyanobacterial origin connects primary plastids with cyanobacteria. Different genes may show variation in the exact evolutionary position, but the cyanobacterial ancestry of primary plastids remains strongly supported.
- Chloroplasts have an outer and inner envelope membrane. A double membrane is compatible with an endosymbiotic origin, but it can not be considered as a single complete proof. Chloroplast DNA, bacterial-related ribosomes, division proteins and molecular phylogenetic evidence together support the endosymbiotic origin much more strongly.
Chloroplast Integration with the Eukaryotic Cell
- During the development of chloroplast from its cyanobacterial ancestor, many genes were transferred from the endosymbiont to the nucleus of the host. This process is known as endosymbiotic gene transfer (EGT).
- The chloroplast genome therefore became highly reduced. Only a limited number of genes remained within the organelle, while many genes required for chloroplast structure and functions are now present in the nuclear genome.
- This transfer created another requirement. The proteins encoded by these nuclear genes are generally synthesized in the cytoplasm but several of them are required inside chloroplast.
- These proteins are transported into the chloroplast by protein-import systems present in its envelope. The TOC and TIC complexes are the major systems associated with transport across the outer and inner chloroplast membranes.
- Modern chloroplast still contains its own DNA, ribosomes, transcription system, translation system and ability to divide. Because of these features, chloroplast is referred to as a semi-autonomous organelle.
- It is not fully independent. Most of the proteins needed for chloroplast development, photosynthesis, metabolism and regulation are encoded by nuclear genes and supplied by the host cell. Thus, during evolution, the chloroplast became strongly dependent on the eukaryotic cell, while still retaining some of its original cyanobacterial machinery.
Chloroplast Function in Photosynthesis
The chloroplast is the site of food synthesis for plant cells, by a mechanism known as photosynthesis. Chlorophyll present in the thylakoids absorbs light energy from the sun. During this process, water and carbon dioxide are converted into organic food with the release of oxygen.
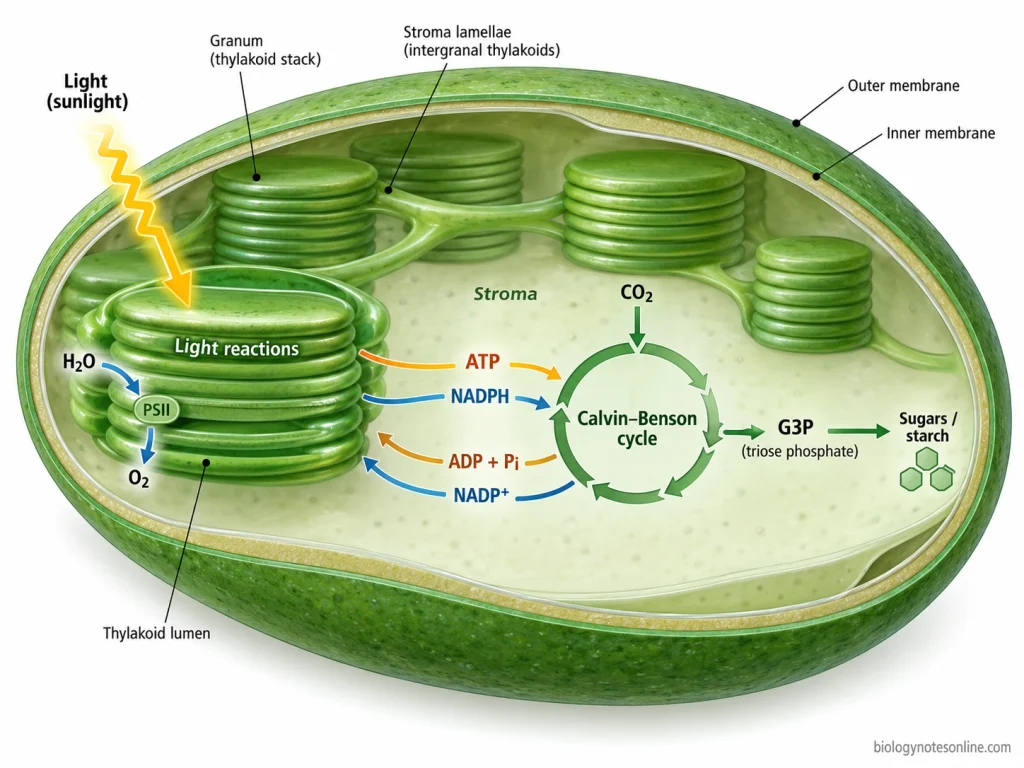
The following are the functions of chloroplast during photosynthesis-
- Trapping of light energy- Thylakoids contain chlorophyll pigments and carotenoids for trapping light energy for use in photosynthesis. This energy is passed into the photosynthetic reaction.
- Splitting of water- In Photosystem II (PSII), water is split and electrons, hydrogen ions (H⁺) and oxygen are formed. Oxygen is released from the plant during this process.
- Movement of electrons- The electrons move through a series of electron carriers in the thylakoid membrane. Energy is released as the electrons pass from one carrier to another, and the electrons finally reach Photosystem I (PSI).
- ATP production- During electron movement, hydrogen ions accumulate inside the thylakoid. These ions then pass through ATP synthase which is used in formation of ATP. This process is referred to as photophosphorylation.
- NADPH formation- In Photosystem I, light energy again raises the energy of electrons. At the end, NADP⁺ takes up the electrons and hydrogen to form NADPH.
- Fixation of carbon dioxide- The ATP and NADPH formed from light reaction are now used in the stroma. Carbon dioxide is fixed with RuBP by the enzyme RuBisCO and enters into the Calvin-Benson cycle.
- Formation of food- During carbon fixation, carbon dioxide is changed into organic carbon compounds. These compounds are further used for manufacturing sugars and starch required by the plant.
Mechanism of Chloroplasts
Chloroplast is a photosynthetic organelle where light energy is converted into chemical energy. The light reaction is carried out in thylakoids and carbon fixation occurs in stroma. Besides these, several synthesis and transport processes also take place in chloroplast.
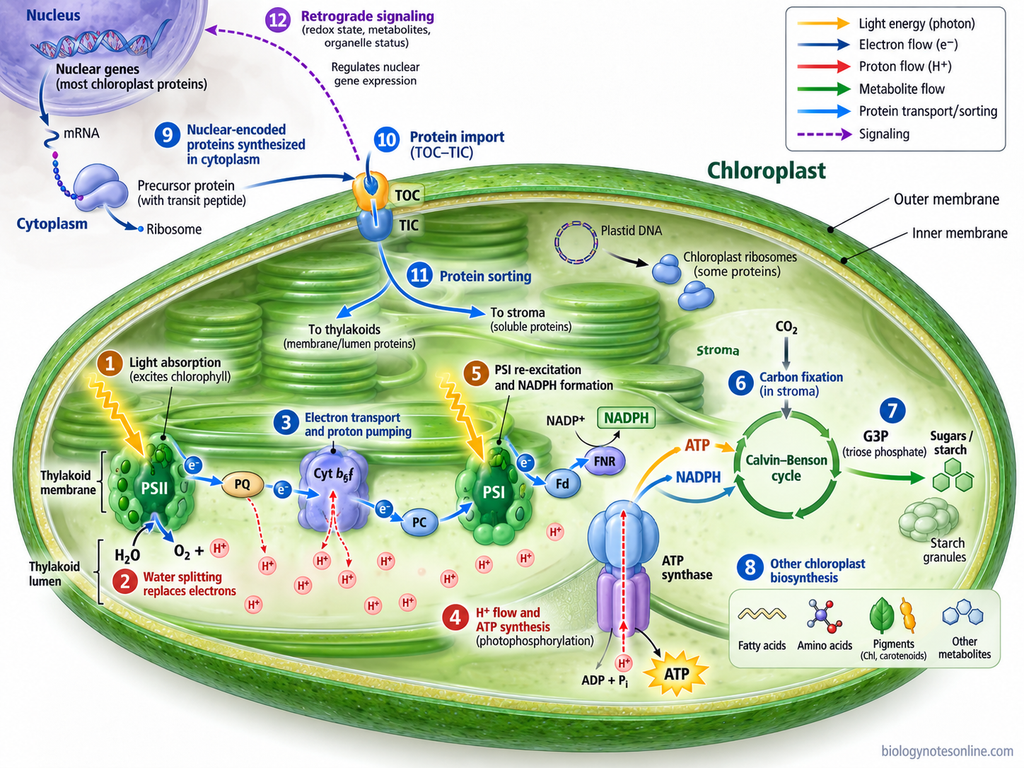
The mechanism takes place in following steps-
- Light is absorbed by chlorophyll and other pigments of the thylakoid membrane. The reaction centre chlorophyll gets excited and electrons are released.
- In Photosystem II (PSII), the lost electrons are replaced by splitting of water molecules. Oxygen, hydrogen ions (H⁺) and electrons are formed during this process.
- The electrons are transferred from PSII through plastoquinone, cytochrome b6f and plastocyanin. At the same time, H⁺ is accumulated inside the thylakoid lumen.
- The accumulated H⁺ moves back through ATP synthase. ATP is formed. This process is referred to as photophosphorylation.
- The electrons now reach Photosystem I (PSI) and again absorb light energy. From PSI they are passed to ferredoxin and finally used for formation of NADPH.
- ATP and NADPH produced in the light reaction are then used in stroma. Here, carbon dioxide is fixed through the Calvin-Benson cycle and converted into organic carbon compounds.
- A part of the fixed carbon is used for sugar formation. Some of it is stored in chloroplast in the form of starch.
- Chloroplast is also a site for different biosynthetic reactions. Fatty acids, amino acids, pigments and several metabolites are synthesized through pathways present in it.
- Most of the proteins required by chloroplast are encoded by nuclear genes. These proteins are synthesized in cytoplasm and not inside the chloroplast.
- The nuclear encoded proteins are brought into chloroplast through TOC and TIC complexes of the envelope.
- After entering chloroplast, the proteins are sent to stroma, thylakoids or other regions according to their function. Some proteins are also synthesized inside chloroplast by its own genetic system.
- Chloroplast can also send signals towards nucleus. Changes in metabolites and redox condition can affect nuclear gene expression. This is referred to as retrograde signaling.
Other Functions of Chloroplast
Besides photosynthesis, chloroplast is involved in several metabolic activities of plant cell. It is the site for synthesis of different cellular compounds, storage of starch and assimilation of some inorganic nutrients. Chloroplast also takes part in signaling and stress responses.
Some of the other functions of chloroplast are-
- Starch storage- A part of the carbon fixed during photosynthesis is stored in chloroplast in the form of starch. This serves as a temporary carbon reserve of the plant.
- Fatty acid synthesis- Chloroplast is an important site for synthesis of fatty acids. These fatty acids are used for formation of different plant lipids.
- Amino acid synthesis- Several amino acids are synthesized through pathways located in chloroplasts. Hence, the function of chloroplast is not limited only to carbohydrate formation.
- Formation of pigments and other compounds- Chlorophyll and carotenoids are synthesized in plastids. Chloroplasts are also involved in formation of several isoprenoid compounds, phytohormones and other metabolites required by the plant.
- Nitrogen assimilation- Inorganic nitrogen is converted into forms that can be incorporated into amino acids and other cellular compounds. Chloroplast takes part in this process.
- Sulfur assimilation- Chloroplast is also involved in assimilation of sulfur. It supplies reduced sulfur compounds for different metabolic activities of plant cell.
- Photorespiration- Chloroplast participates in photorespiration along with peroxisomes and mitochondria. During this process, compounds produced by the oxygenase activity of RuBisCO are further metabolized and part of the carbon is recovered.
- Cell signaling and stress response- Chloroplast can produce different signals according to its metabolic and physiological condition. Some of these signals are passed to the nucleus and regulate nuclear gene expression. This is referred to as retrograde signaling. It is also associated with plant responses to high light, drought, heat and other stresses.
References
- Chan, K. X., Crisp, P. A., Estavillo, G. M., & Pogson, B. J. (2010). Chloroplast-to-nucleus communication: Current knowledge, experimental strategies and relationship to drought stress signaling. Plant Signaling & Behavior, 5(12), 1575–1582. https://doi.org/10.4161/psb.5.12.13758
- Chen, C., MacCready, J. S., Ducat, D. C., & Osteryoung, K. W. (2018). The molecular machinery of chloroplast division. Plant Physiology, 176(1), 138–151. https://doi.org/10.1104/pp.17.01272
- Cooper, G. M. (2000). The cell: A molecular approach (2nd ed.). Sinauer Associates. https://www.ncbi.nlm.nih.gov/books/NBK9839/
- Eckardt, N. A. (2005). Photorespiration revisited. The Plant Cell, 17(8), 2139–2141. https://doi.org/10.1105/tpc.105.035873
- Johnson, M. P. (2016). Photosynthesis. Essays in Biochemistry, 60(3), 255–273. https://doi.org/10.1042/EBC20160016
- Li, B., Kronzucker, H. J., & Shi, W. (2013). Molecular components of stress-responsive plastid retrograde signaling networks and their involvement in ammonium stress. Plant Signaling & Behavior, 8(2), e23107. https://doi.org/10.4161/psb.23107
- Li, J.-Y., Yang, C., Tian, Y.-Y., & Liu, J.-X. (2022). Regulation of chloroplast development and function at adverse temperatures in plants. Plant and Cell Physiology, 63(5), 580–591. https://doi.org/10.1093/pcp/pcac022
- Li, M., & Kim, C. (2022). Chloroplast ROS and stress signaling. Plant Communications, 3(1), 100264. https://doi.org/10.1016/j.xplc.2021.100264
- Malinova, I., Qasim, H. M., Brust, H., & Fettke, J. (2018). Parameters of starch granule genesis in chloroplasts of Arabidopsis thaliana. Frontiers in Plant Science, 9, 761. https://doi.org/10.3389/fpls.2018.00761
- Ostermeier, M., Garibay-Hernández, A., Holzer, V. J. C., Schroda, M., & Nickelsen, J. (2024). Structure, biogenesis, and evolution of thylakoid membranes. The Plant Cell, 36(10), 4014–4035. https://doi.org/10.1093/plcell/koae102
- Pyke, K. (2009). Plastid biology. Cambridge University Press. https://doi.org/10.1017/CBO9780511626715
- Renna, L., Papini, A., Mancuso, S., Brandizzi, F., & Stefano, G. (2026). Plant plastids: From evolutionary origins to functional specialization and organelle interactions. Journal of Experimental Botany, 77(1), 63–85. https://doi.org/10.1093/jxb/eraf378
- Richardson, L. G. L., & Schnell, D. J. (2020). Origins, function, and regulation of the TOC–TIC general protein import machinery of plastids. Journal of Experimental Botany, 71(4), 1226–1238. https://doi.org/10.1093/jxb/erz517
- Sabater, B. (2018). Evolution and function of the chloroplast: Current investigations and perspectives. International Journal of Molecular Sciences, 19(10), 3095. https://doi.org/10.3390/ijms19103095
- Sakamoto, W., Miyagishima, S.-Y., & Jarvis, P. (2008). Chloroplast biogenesis: Control of plastid development, protein import, division and inheritance. The Arabidopsis Book, 6, e0110. https://doi.org/10.1199/tab.0110
- Song, Y., Feng, L., Alyafei, M. A. M., Jaleel, A., & Ren, M. (2021). Function of chloroplasts in plant stress responses. International Journal of Molecular Sciences, 22(24), 13464. https://doi.org/10.3390/ijms222413464
- Sun, A.-Z., & Guo, F.-Q. (2016). Chloroplast retrograde regulation of heat stress responses in plants. Frontiers in Plant Science, 7, 398. https://doi.org/10.3389/fpls.2016.00398
- Ünal, D., García-Caparrós, P., Kumar, V., & Dietz, K.-J. (2020). Chloroplast-associated molecular patterns as concept for fine-tuned operational retrograde signalling. Philosophical Transactions of the Royal Society B: Biological Sciences, 375(1801), 20190443. https://doi.org/10.1098/rstb.2019.0443
- Zhao, C., Haigh, A. M., Holford, P., & Chen, Z.-H. (2018). Roles of chloroplast retrograde signals and ion transport in plant drought tolerance. International Journal of Molecular Sciences, 19(4), 963. https://doi.org/10.3390/ijms19040963
- Zoschke, R., & Bock, R. (2018). Chloroplast translation: Structural and functional organization, operational control, and regulation. The Plant Cell, 30(4), 745–770. https://doi.org/10.1105/tpc.18.00016
미토콘드리아는 어머니를 통해, 다른 생명에 전달되는데, 독립 세포인 엽록체는 어떻게 다음 세대 나무에게 이동하나요?
미토콘드리아는 실제로 인간을 포함한 대부분의 유기체에서 어머니에서 자손으로 전달됩니다. 이 과정은 엽록체를 포함하는 식물과 기타 광합성 유기체에서는 약간 다릅니다.
엽록체는 미토콘드리아와 마찬가지로 식물과 조류의 세포에서 발견되는 세포 소기관입니다. 그들은 빛 에너지가 화학 에너지로 변환되는 과정인 광합성을 담당합니다. 엽록체의 유전은 종에 따라 달라질 수 있습니다.
대부분의 식물에서 엽록체는 동물의 미토콘드리아와 유사하게 모계를 통해 유전됩니다. 이는 엽록체가 일반적으로 모식물의 밑씨에 있는 난세포를 통해 자손에게 전달된다는 것을 의미합니다. 수정 과정에서 (아버지 식물에서 나온) 꽃가루의 정자 세포는 핵 DNA만 접합체에 제공하고 엽록체와 같은 세포소기관에는 제공하지 않습니다. 결과적으로 자손의 엽록체는 일반적으로 모식물의 엽록체와 유전적으로 동일합니다.
그러나 이 규칙에는 예외가 있습니다. 일부 식물에서는 엽록체가 아버지 또는 부모 모두로부터 물려받을 수 있습니다. 엽록체의 이러한 부계 또는 양부모 유전은 덜 일반적이지만 특정 종에서 관찰되었습니다.